Ask questions across claims linked to experiments, exact results, limitations, and sources.Know what falsifiable science actually supports before you trust the answer.
Press Enter ↵ to search evidence
Explore by Goal
"Mood reflects the biology of the brain. How you feel is affected by the chemicals in the brain, and these are the same chemicals that form the basis of mood-altering drugs."
- Liz Miller
Quick Explanation
Copied
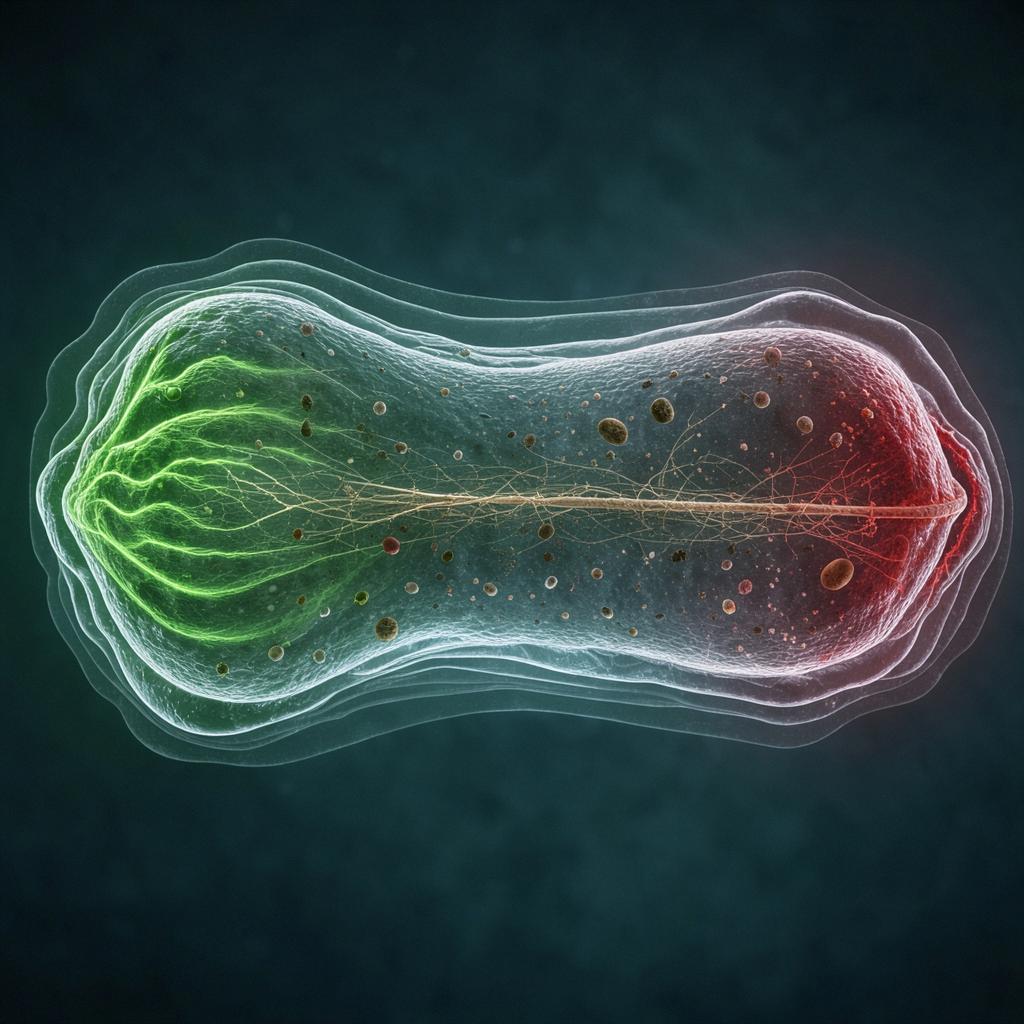
This Bulletin of Mathematical Biology paper by Buttenschön, Liu, and Edelstein-Keshet extends 1D wave-pinning theory to dynamically growing/shrinking cells with Kelvin-Voigt mechanics, analytically proving invariant regions and steady-state counts, and numerically revealing dilution-induced oscillations, size-dependent loss of polarity, and rich Rac–Rho motility behaviors .
Long Explanation
What the Paper Claims and How Well It Supports It
The paper generalizes the 1D wave-pinning model of Mori et al. (2008) to a cell whose length L(t) changes, using a correct mass balance on a deforming domain (Crampin-style reaction–transport–diffusion equation) mapped onto the fixed interval [-1, 1]. The transformation introduces a dilution term −(Ṙ/R)·u and a time-dependent diffusion coefficient D/R²(t), and eliminates advection — a clean, pedagogically valuable result derived in the appendices .
The strongest analytical contributions are: (1) proof that the region Ω = {L > 0, G ≥ 0, G ≤ GT/L} is invariant under the coupled mechanics–signaling ODE flow; (2) a Descartes-rule argument that the reduced system has 1 or 3 positive steady states under sharp-switch approximation; and (3) full linear stability plus AUTO bifurcation analysis showing tristability in the contractile (Rho) case and stable limit cycles (Hopf bifurcations) only in the protrusive (Rac) case — the basis of the paper's headline "dilution-induced oscillations" result .
Full spatiotemporal simulations (finite differences, ROWMAP stiff integrator, tolerance 10⁻⁶) then show: polarity is lost if the cell grows or shrinks too much (both extremes exit the wave-pinning regime); soft cells depolarize because mechanical restoration is slower than signaling collapse; Rac fronts drive motion, Rho contraction can generate push-based "squeezing" motility; and the mutually antagonistic Rac–Rho model yields metastable bipolar states, stalling, and delayed motility onset depending only on initial conditions .
Reported parameter ranges only — no simulated values. The wide spans (e.g., μ and Fmax spanning two orders of magnitude) signal substantial parameter uncertainty inherited from 3D literature sources.
Critical Assessment: Strengths, Blind Spots, and Falsifiability
Strengths: rare combination of rigorous analysis (invariant region, Descartes rule, stability classification) with accessible numerics; honest acknowledgment that the force law F(G) = ±FmaxGm/(Gcm+Gm) is "simply one case we chose to analyze"; and a constant-volume variant (Appendix D) tested to check robustness of the dilution assumption. The rest-length vs. end-force equivalence is proven, unifying with Zmurchok et al. (2018).
Blind spots and limitations the authors partially acknowledge: (a) the 1D transect geometry limits contact with real cell shape — 2D extension is deferred as future work; (b) the proportional membrane/cytosol scaling assumption is only exact in confined channels; (c) no experimental validation whatsoever — every "dilution-induced oscillation" and depolarization threshold is a model prediction awaiting testing (e.g., against micropatterned or confinement experiments of the kind in Holmes et al. 2012); (d) mechanical parameters are borrowed from 3D multicellular models (Drasdo, Palsson), an under-justified transfer to a single-cell 1D problem; (e) parameters such as Hill coefficients n up to 25 and 1000-fold diffusion ratios were chosen partly for mathematical convenience ("sufficiently large regime in which oscillations are possible"), which risks tuning the model toward interesting behavior; (f) no public code/data repository is stated, though the methods (ROWMAP, N = 2¹⁰ grid, f2py wrappers) are described in enough detail to reimplement; (g) the two-GTPase uniform analysis is admittedly preliminary (nine possible equilibria, only "preliminary exploration"), so conclusions there are weaker than the single-GTPase results.
Confidence note: the analytical claims are internally consistent and standard-method based (moderate-to-strong confidence); the biological relevance of specific parameter regimes and the transient dynamics emphasized in Fig. 9 remain genuinely uncertain until validated. The paper itself flags transient dynamics — not just asymptotics — as an open, urgent problem. Falsification would require experiments showing wave-pinning persistence across large size excursions, or absence of size-triggered depolarization in soft cells.
Feedback:
Updated: November 17, 2026
BGPT Paper Review
Study Novelty
80%
First full coupling of spatially distributed (non-uniform) GTPase wave-pinning dynamics with deforming-domain dilution and viscoelastic mechanics; dilution-induced Rac oscillations and size-triggered depolarization are genuinely new in this minimal framework, though built on well-established prior scaffolding (Mori 2008, Holmes & Edelstein-Keshet 2016, Zmurchok 2018).
Scientific Quality
80%
Rigorous proofs (invariant region, Descartes rule, stability), proper bifurcation software (AUTO), and a robustness appendix. Deductions for zero experimental validation, parameters borrowed from 3D models, and Hill coefficients chosen partly to enlarge the oscillatory regime.
Study Generality
70%
The dilution-coupled wave-pinning framework applies broadly to polarity systems and growing domains, but restriction to 1D geometry and single/mutual-inhibition GTPase kinetics narrows direct biological generality until 2D/3D extensions exist.
Study Usefulness
80%
Provides a reusable minimal framework, exact transformations, and testable predictions (depolarization at size extremes, oscillation regimes, stiffness thresholds) that experimental cell-polarity groups and computational modelers can directly use; no code repository limits immediate reuse.
Study Reproducibility
70%
Methods are detailed (ROWMAP integrator, N=2^10 grid, tolerance 10^-6, full parameter tables), and numerical tools are public; however, no deposited code or dataset, and some parameter choices span wide unspecified ranges.
Explanatory Depth
90%
Deep mechanistic explanation: dilution term derived from first principles, steady states characterized in closed form under sharp-switch limits, Hopf bifurcations classified, and behavioral regimes mapped in two-parameter bifurcation diagrams.
We'll email you the results when your analysis is finished.
Hypothesis Graveyard
Dilution alone (without mechanics) explains polarity loss — refuted by the paper's own shrinking-domain simulations, where both growth and shrinkage independently exit the wave-pinning regime via the bifurcation structure, not dilution per se.
A nonlinear spring is required for oscillations (Dierkes et al. 2014) — superseded here: linear Kelvin-Voigt mechanics plus saturating GTPase-dependent forces suffice to generate Hopf bifurcations.

 Explore by Goal
 Quick Explanation
 Long Explanation
 Top Data Sources
 Ask a Follow-Up
 Key Insight
 Keep Exploring
 Hypothesis Graveyard
 Potential Experiments
 Discussion
